
Pinball1970
Valued Senior Member


These pages (I had to load copy and store them as images so I could rotate them to read them) seem to be just a description of the handicap principle. I saw no comment on whether Dawkins thinks it is valid.This edition.
View attachment 7736


Handicap principle - Wikipedia
en.wikipedia.org
These pages (I had to load copy and store them as images so I could rotate them to read them) seem to be just a description of the handicap principle. I saw no comment on whether Dawkins thinks it is valid.
We've always recognized that signals can actually be handicaps. We understood that, in the process of evolution, especially through sexual selection, extreme handicaps can arise, despite the fact that they are handicaps. Part of Zahavi's theory that we objected to was the idea that selection might favor certain signals precisely because they are handicaps for those who use them. Alan Grafen clearly rehabilitates this very point. If Grafen is right (and I think he is), this result has significant implications for the entire study of animal signals. It may require fundamental changes in our views on the evolution of behavior and on many of the issues discussed in this book. Sexual advertising is only one kind of advertising. The Zahavi-Graefen theory, if correct, will upend biologists' understanding of the relationships between rivals of the same sex, between parents and offspring, and between enemies of different species. This prospect unnerved me somewhat, because it means that it will no longer be possible to dismiss almost insane theories from the standpoint of common sense. If we see an animal genuinely behaving stupidly, for example, standing on its head when it sees a lion, it may be doing so to show off for a female. It may even be showing off for the lion: "I'm such a high-quality animal that trying to catch me is just a waste of time."
He said it could become an ESS, exist in nature. I'll try and scan in another page after work.These pages (I had to load copy and store them as images so I could rotate them to read them) seem to be just a description of the handicap principle. I saw no comment on whether Dawkins thinks it is valid.
What's an ESS?He said it could become an ESS, exist in nature. I'll try and scan in another page after work.
Images is a pain on this device.
Evolutionary Stable Strategy, John Maynard Smith analysis of different genetic combinations in populations.What's an ESS?
Scanned text are hard to read. Maybe my citation above is sufficient? Dawkins wrote that he understood that the "common sense" can be wrong, "insane" theories can be true and this is even nerving. This is what I tried to explain in this thread.I'll try and scan in another page after work.

 www.scienceforums.net
Well that makes sense but doesn't account for why these instances of flashy bling do nevertheless occasionally arise, which is presumably what the Handicap hypothesis was intended to explain. So what is now the accepted explanation for those? Is it just like genetic drift, i.e. something that rises by accident and is tolerated by natural selection if it does not unduly impede breeding success?The chat over at Dot Net may be helpful in getting through some of the conceptual challenges of honest signalling, finding optimal balance between costs of display and viability, etc.
The handicap principle
(I don't want to paste in everything Seth, Charon, and I wrote over there)
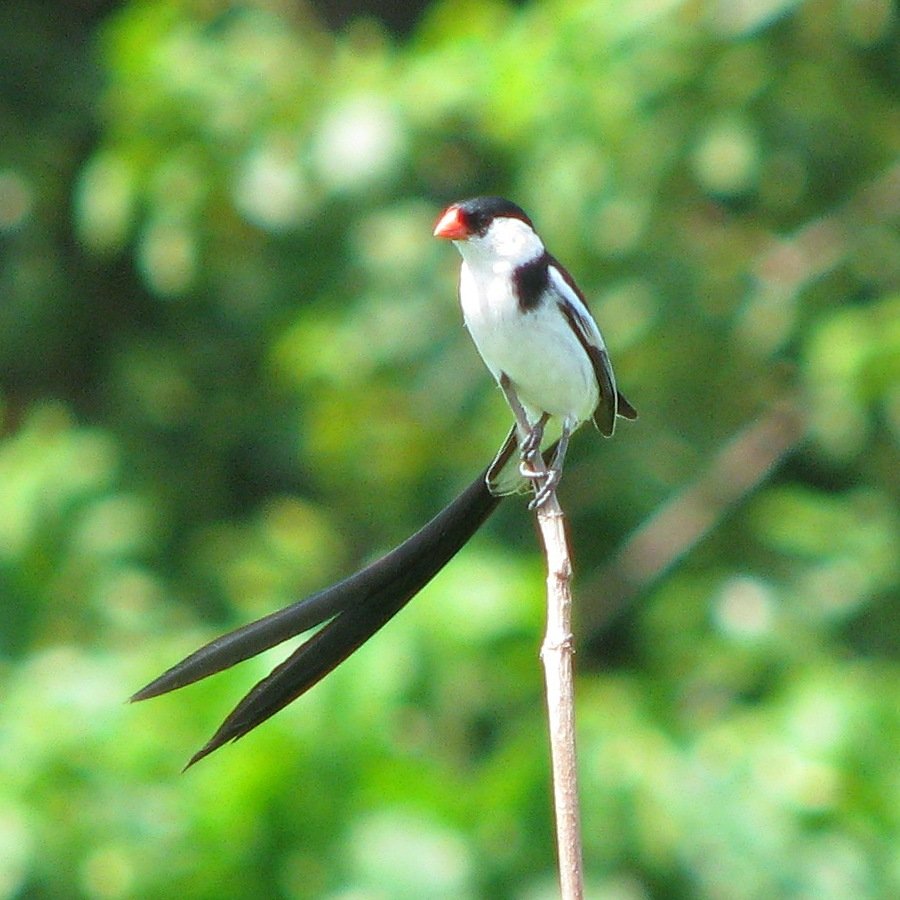
Basically, the theories move now towards seeing that equilibrium between display costs (metabolic, hazard, social, etc) and viability are not necessarily about waste. Index signalling, for example, is not wasteful, since it comes from basic physiology and morphology of the animal and not conspicuous and expensive alterations during mating season. Stotting gazelles can jump high because they are built for it and it's useful for seeing farther around them and a side benefit of having powerful legs. It doesn't drain their metabolic funds or incur other costs. It's an honest display of vigor, also can be adapted for courtship displays. Natural selection will tend more towards stotters than peacocks with pounds of arse plumage. Handicapping is atypical because natural selection pressures towards overall viability in environments that are unforgiving of over-investment in flashy bling.
I would have to flatten the book and damage the pristine spine.Scanned text are hard to read. Maybe my citation above is sufficient? Dawkins wrote that he understood that the "common sense" can be wrong, "insane" theories can be true and this is even nerving. This is what I tried to explain in this thread.
Yes, males in species that practice, say, brood parasitism are going to have more leeway to wear themselves out in courting behavior and mating. So maybe they can drift into more extravagant investments which reduce their own viability, while still edging out weaker males. "Drift" might not be inaccurate in that it's tolerated by NS where over-investment doesn't affect an ecosystem by reducing overall food supply or disrupting communication networks, etc. Interesting point about how female aesthetics can shift in ways that are selectively neutral (while presumably attraction is still anchored in primary index signals of health and strength....a female could see two males who can both lift 15 pounds of tail feathers off the ground and know both are strong, but then pick one on the basis of a gaudier purple bib).Well that makes sense but doesn't account for why these instances of flashy bling do nevertheless occasionally arise, which is presumably what the Handicap hypothesis was intended to explain. So what is now the accepted explanation for those? Is it just like genetic drift, i.e. something that rises by accident and is tolerated by natural selection if it does not unduly impede breeding success?
I can imagine there could be irrelevant features that happen to appeal aesthetically to females, due to some side effect of how their brains are wired, which won't be weeded out by natural selection so long as (1) the males live long enough to impregnate the females and (2) the males are not required to take part in rearing the young after mating - or are not impeded by the feature in question in doing so.
The Y chromosome has few genes that would be linked to "traits."these would be traits encoded on the Y
No. And most genes do not express as simple specific phenotypic traits. For example, male baldness is mediated by over 250 gene loci and most of them are autosomal.A question for those familiar with Grafen’s experiment: am I right that the "handicaps" (inherently disadvantageous traits that help a male attract females precisely because they are disadvantageous) are exclusively male traits that aren't passed on to female offspring?
I suppose, this is of no importance? For example, there is no single gene defining the size of ... for men, but anyway all the genes which define it, are located in Y chromosome.No. And most genes do not express as simple specific phenotypic traits. For example, male baldness is mediated by over 250 gene loci and most of them are autosomal.
Already said there are few genes that would contribute to a trait on that Chromosome.I suppose, this is of no importance? For example, there is no single gene defining the size of ... for men, but anyway all the genes which define it, are located in Y chromosome.
No. You are missing the point. The main function of the Y chromosome is to switch on a whole series of other genes, related to male characteristics, that are located elsewhere.I suppose, this is of no importance? For example, there is no single gene defining the size of ... for men, but anyway all the genes which define it, are located in Y chromosome.
